Uncommon Descent Serving The Intelligent Design Community

Interesting proteins: DNA-binding proteins SATB1 and SATB2

Categories
Intelligent Design
Share
Facebook
Twitter/X
LinkedIn
Flipboard
Print
Email

With this OP, I am starting a series (I hope) of articles whose purpose is to present interesting proteins which can be of specific relevance to ID theory, for their functional context and evolutionary history.

DNA-binding protein SATB1

SATB1 (accession number Q01826) is a very intriguing molecule. Let’s start with some information we can find at Uniprot, a fundamental protein database, about what is known of its function (in the human form):

Crucial silencing factor contributing to the initiation of X inactivation mediated by Xist RNA that occurs during embryogenesis and in lymphoma

And:

Transcriptional repressor controlling nuclear and viral gene expression in a phosphorylated and acetylated status-dependent manner, by binding to matrix attachment regions (MARs) of DNA and inducing a local chromatin-loop remodeling. Acts as a docking site for several chromatin remodeling enzymes

IOWs, it is an important regulatory protein involved in many different, and not necessarily well understood, processes, which binds to DNA and in involved in chromatin remodeling.

It is also involved in hematopoiesis (especially in T cell development), and has important roles in the biology of some tumors:

Modulates genes that are essential in the maturation of the immune T-cell CD8SP from thymocytes. Required for the switching of fetal globin species, and beta- and gamma-globin genes regulation during erythroid differentiation. Plays a role in chromatin organization and nuclear architecture during apoptosis.

Reprograms chromatin organization and the transcription profiles of breast tumors to promote growth and metastasis.

Keywords for molecular function: Chromatin regulator, DNA-binding, Repressor

Now, some information about the protein itself. I will relate, again, to the human form of the protein:

Length: 763 AAs. It’s a rather big protein, like many important regulatory molecules.

Its subcellular location is in the nucleus.

It is a multi-domain protein, with at least 5 detectable domains and many DNA binding sites.

Evolutionary history of SATB1

Now, let’s see some features of the evolutionary history of this protein in the course of metazoa evolution.

I will use here the same tools that I have developed and presented in my previous OP:

The amazing level of engineering in the transition to the vertebrate proteome: a global analysis

So, I invite all those who are interested in the technical details to refer to that OP.

Here is a graph of the levels of homology to the human protein detectable in other metazoan groups, expressed as mean bitscore per aminoacid site:


Fig. 1: Evolutionary history of SATB1 by human-conserved functional information
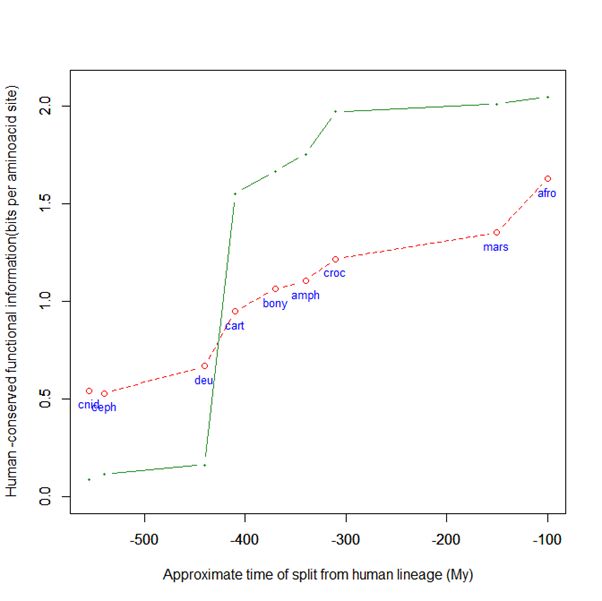
 

The green line represents the evolutionary history of our protein, while the red dotted line is the reference mean line for the groups considered, as already presented in my previous post quoted above (Fig. 2).

As everyone can see, this specific protein has a very sudden gain in human-conserved information with the transition from pre-vertebrates to vertebrates. So, it represents a very good example of the information jump that I have tried to quantify globally in my previous post.

Here, the jump is of almost 1.5 bits per aminoacid site. What does that mean?

Let’s remember that the protein is 763 AA long. Therefore, an increase of information of 1.5 bits per aminoacid corresponds to more than 1000 bits of information. To be precise, the jump from the best pre-vertebrate hit to the best hit in cartilaginous fish is:

1049 bits

But let’s see more in detail how the jump happens.

I will show here in detail some results of protein blasts. All of them have been obtained using the Blastp software at the NCBI site:

https://blast.ncbi.nlm.nih.gov/Blast.cgi?PROGRAM=blastp&PAGE_TYPE=BlastSearch&LINK_LOC=blasthome

with default settings.

Here is the result of blasting the human protein against all known protein sequences except for vertebrate sequences:

Fig. 2: Results of blasting human SATB1 against all non vertebrate protein sequences
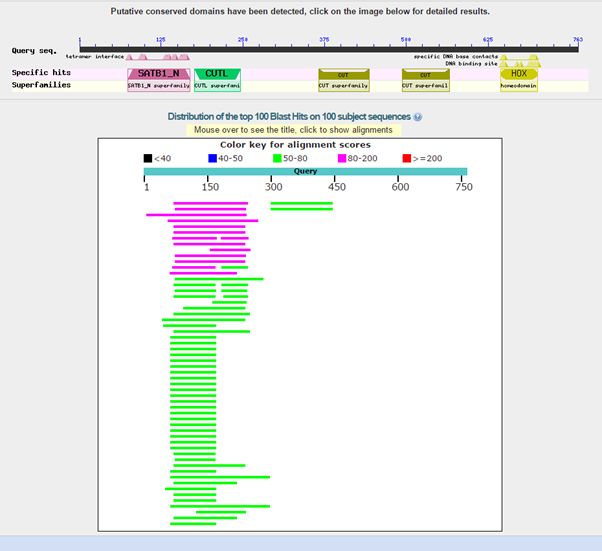
 

As can be seen, we find only low homologies in non vertebrates, and they are essentially restricted to a small part of the molecule, that correspond to the first two domains in the protein, or just to the first domain. The image shows clearly that all the rest of the sequence has no detectable significant homologies in non vertebrates (except for a couple of very low homologies for the third domain).

The best hit in non vertebrates is 154 bits with Parasteatoda tepidariorum, a spider. Here it is:

Fig. 3: The best hit in non vertebrates (with a spider)
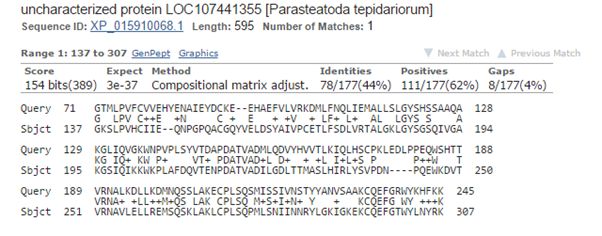
The upper line (Query) is the human sequence. The bottom line (Sbjct) is the aligned sequence of the spider. In the middle line, letters are identities, “+” characters are similarities (substitutions which are frequently observed in proteins, and are probably quasi-neutral), and empty spaces are less frequent substitutions, those that are more likely to affect protein structure and function if they happen at a functionally important aminoacid site.

The alignment here is absolutely restricted to AAs 71 – 245 (the first two domains), and involves only 177 AAs. Of these, only 78 (44%) are identities and 111 (62%) are positives (identities + similarities). So, in the whole protein we have only 78 identities out of 763 (10.2%).

The spider protein is labeled as “uncharacterized protein”, and that is the case in most of the other non vertebrate hits.

All the other non vertebrate hits, with a couple of exceptions, are well below 100 bits, most of them between 70 and 86 bits.

IOWs, the protein as we know it in vertebrates essentially does not exist in non vertebrates.

Even non vertebrate deuterostomia, which should be the nearest precursors of the first vertebrates, have extremely low homology bitscores with the human protein:

Saccoglossus kowalevskii (hemichordates):  87 bits

Branchiostoma floridae (cephalochordate): 67 bits

The information jump in vertebrates

Now, what happens with the first vertebrates?

The oldest split in vertebrates is the one between cartilaginous fish and bony fish (from which the human lineage derives). Therefore, homologies that are conserved between cartilaginous fish and humans had reasonably to be already present in the Last Common Ancestor of Vertebrates, before the split between cartilaginous fish and bony fish, and have been conserved for about 420 million years.

So, let’s see the best hit between the human protein and cartilaginous fish. It is with Rhincodon typus (whale shark). Here it is:


Fig. 4: The best hit of human SATB1 in cartilaginous fish (with the whale shark)
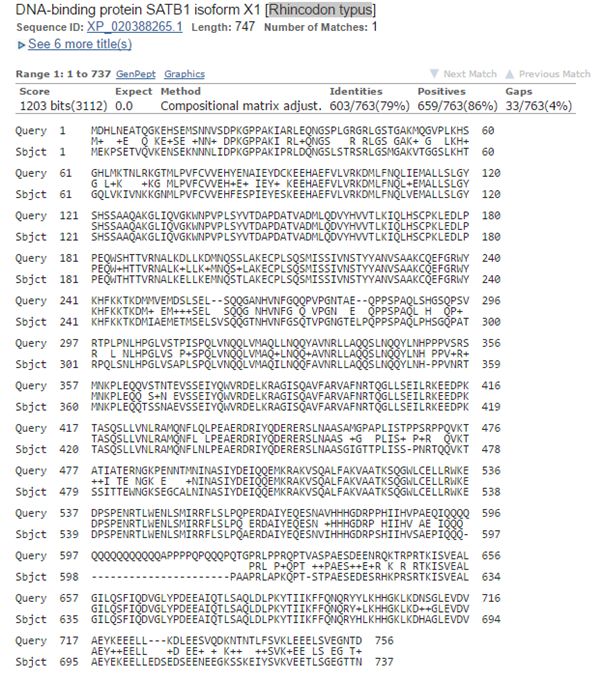
 

Here, the alignment involves practically the whole molecule (756 AAs), and we have 1203 bits of homology, 603 identities (79%), 659 positives (86%).

IOWs, the two molecules are almost identical. And the homology is extremely high not only in the domain parts, but also in the rest of the protein sequence.

Now, the evolutionary time between pre-vertebrates and the first split in vertebrates is certainly rather small, a few million years, or at most 20 – 30 million years. Not a big chronological window at all, in evolutionary terms.

However, in that window, this protein appears almost complete. 603 aminoacids are already those that will remain up to the human form of the protein, and only 78 of them were detectable in the best hit before vertebrate appearance.

1049 bits of new, original functional information. In such a short evolutionary window.

Functionality

Why functional? Because those 603 aminoacid have remained the same thorugh more than 400 million years of evolution. They have evaded neutral or quasi neutral variation, that would have certainly completely transformed the sequence in such a big evolutionary time, if those aminoacid sites were not under extreme functional constraint and purifying (negative) selection.

Now, I say that this fact cannot in any way be explained by any neo-darwinian model. Absolutely not.

Moreover, there is absolutely no evidence in the available proteome of any intermediate form, of any gradual development of the functional sequence that will be conserved up to humans (except, of course, for the 50 – 78 AAs which are already detectable in the first two domains in many pre -vertebrates).

By the way, Callorhincus milii, the Elephant shark, has almost identical values of homology:

1184 bits, 599 identities, 654 positives

But, how important is this protein?

In the ExAC database, a database of variations in the human genome, missense mutations are 110 out of 260.3 expected, with a z score of 4.56, an extremely high measure of functional constraint.

The recent medical literature has a lot of articles about the important role of SATB1 at least in two big fields:

  • T cell development
  • Tumor development (many different kinds of tumors)

If we want to sum up in a few words what is known, we could say that SATB1 is considered a master regulator, essentially a complex transcription repressor, involved mainly (but not only) in the development of the immune system, in particular T cells. A disregulation of this protein is linked to many aspects of tumor invasivity (especially metastases). The protein seems to act, among other possibilities, as a global organizer of chromatin states.

Here is a very brief recent bibliography:

Essential Roles of SATB1 in Specifying T Lymphocyte Subsets

SATB1 overexpression correlates with gastrointestinal neoplasms invasion and metastasis: a meta-analysis for Chinese population

SATB1-mediated Functional Packaging of Chromatin into Loops

DNA-binding protein SATB2

But there is more. There is another protein which is very similar to SATB1. It is called DNA-binding protein SATB2 (accession number Q9UPW6).

Its length is very similar to SATB1: 733 AAs.

Uniprot describes its function as follows:

Binds to DNA, at nuclear matrix- or scaffold-associated regions. Thought to recognize the sugar-phosphate structure of double-stranded DNA. Transcription factor controlling nuclear gene expression, by binding to matrix attachment regions (MARs) of DNA and inducing a local chromatin-loop remodeling. Acts as a docking site for several chromatin remodeling enzymes

Which is very similar to SATB1. But now come the differences. While SATB1 is implied prevalently in T cell development and tumor development, SATB2 is:

Required for the initiation of the upper-layer neurons (UL1) specific genetic program and for the inactivation of deep-layer neurons (DL) and UL2 specific genes, probably by modulating BCL11B expression. Repressor of Ctip2 and regulatory determinant of corticocortical connections in the developing cerebral cortex. May play an important role in palate formation. Acts as a molecular node in a transcriptional network regulating skeletal development and osteoblast differentiation

So, similar proteins with rather different specificities. While SATB1 is mainly connexted to adaptive immunity (T cell development), SATB2 seems to be more linked to neuronal development. Like SATB1, it is involved in cancer development, although usually in different types of cancer.

Here is a brief recent bibliography about SATB2:

Mutual regulation between Satb2 and Fezf2 promotes subcerebral projection neuron identity in the developing cerebral cortex

SATB1 and SATB2 play opposing roles in c-Myc expression and progression of colorectal cancer

However, how similar is SATB2 to SATB1 in terms of sequence homology?

Here is a direct blast of the two human molecules:


Fig. 5: Blast of human SATB1 vs human SATB2:
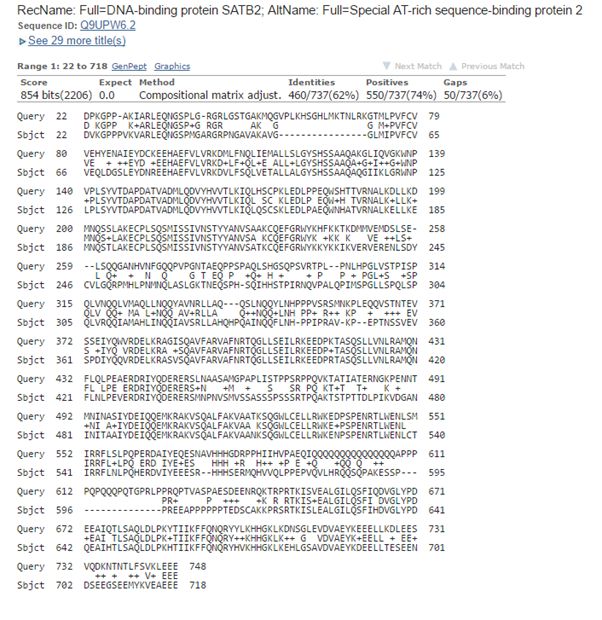
 

OK, they are very similar, but…  only 460 identities, 550 positives, 854 bits. IOWs, these two human proteins are similar, but not so similar as the two sequences of SATB1 in the shark and in humans.

Now, here is the evolutionary history of SATB2:


Fig. 6: Evolutionary history of SATB2 by human-conserved functional information
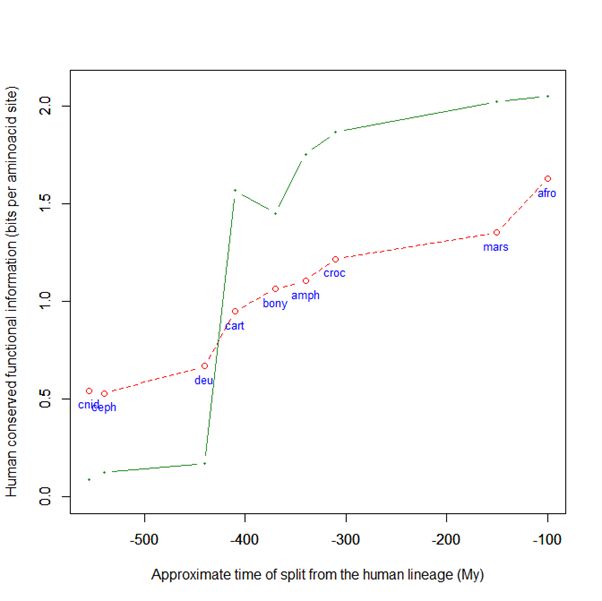
 

As everyone can see, it is almost identical to the evolutionary history of SATB1. To see it even better, Fig. 7 shows the two evolutionary histories together (the green line is SATB1, the brown line is SATB2):


Fig. 7: Evolutionary history of SATB1 and SATB2 by human-conserved functional information
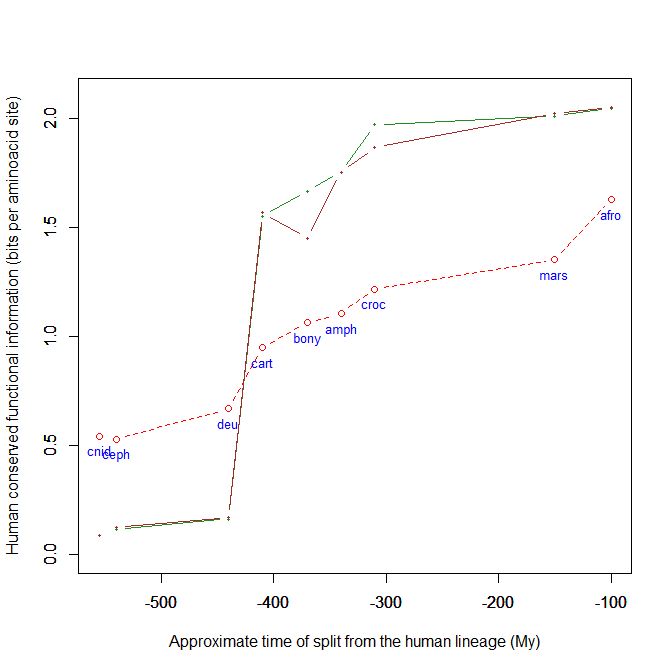
 

In particular, pre-vertebrate history and the jump in cartilaginous fish are practically identical. And yet these are two different molecules, as we have seen, with different specificities and about one third of difference in sequence.

Now, let’s blast human SATB2 against cartilaginous fish. Again the best hit is with the whale shark:


Fig. 8: The best hit of human SATB2 in cartilaginous fish (with the whale shark)
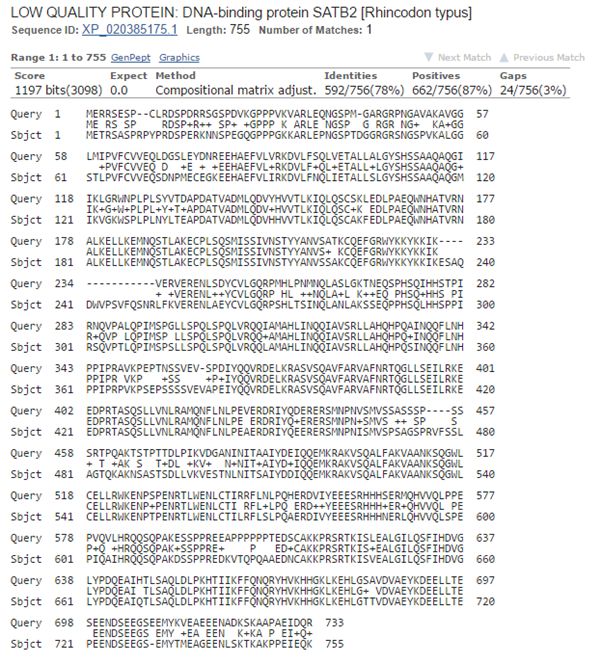
 

And the numbers are very similar, incredibly similar I would say, to those we found for SATB1:

1197 bits, 592 identities, 662 positives.

But what if we blast SATB1 of the whale shark against SATB2 of the whale shark?

Here are the results:


Fig. 9: Blast of whale shark SATB1 vs whale shark SATB2:
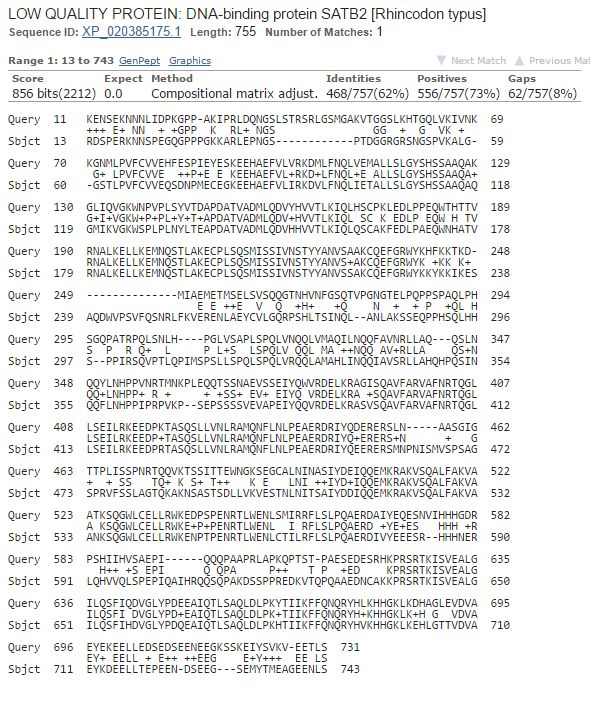
Now, please, compare the numbers we got here with those from the similar blast between the two proteins in humans:

SATB1 human vs SATB2 human:  460 identities, 550 positives, 854 bits

SATB1 shark vs SATB2 shark:      468 identities, 556 positives, 856 bits

Almost exactly the same numbers! Wow!

What does that mean?

It means that this system of two similar proteins with different function arises in vertebrates as a whole system, already complete, with the two components already differentiated, and is conserved almost identical up to humans. Indeed, SATB1 and SATB2 have the same degree of homology both in sharks and in humans, and the two SATB1 proteins in shark and humans, as well as the two SATB2 proteins in shark and humans, have greater similarity, after more than 400 million years of divergence, than SATB1 and SATB2 show when compared, both in sharks and in humans.

Would you describe that as sudden appearance of huge amounts of functional information, followed by an extremely long stasis? I certainly would!

The following table sums up these results:

Sequence 1 Sequence 2 Bitscore
SATB1 Human SATB2 Human 854
SATB1 Shark SATB2 Shark 856
SATB1 Human SATB1 Shark 1203
SATB2 Human SATB2 Shark 1197

IOWs, the whole system appeared practically as it is today, before the split of cartilaginous fish and bony fish, and has retained its essential form up to now.

So, the total amount of new functional information implied by the whole system of these two proteins is about 1545 bits (considering 855 bits of common information, and 345 bits x 2 of specific information in each molecule).

An amazing amount, for a system of just two molecules, considering that 500 bits is Dembski’s Universal Probability Bound!

Let’s remember that in my previous post, quoted above, I showed that the informational jump from pre-vertebrates to vertebrates is more than 1.7 million bits. That’s a very big number, but big numbers sometimes are not easily digested. So, I believe that seeing that just two important molecules can contribute for almost 1500 bits can help us understand what we are really seeing here.

Moreover, it’s certainly not a case that those two molecules seem to be fundamental in two very particular fields:

a) The adaptive immune system

b) The nervous system

if we consider that those are exactly the two most relevant developments in vertebrates.

And, as a final note, please consider that these are very complex master regulators, which interact with tens of other complex proteins to effect their functions. The whole system is certainly much more irreducibly complex than we can imagine.

But still, just the analysis of these two sister proteins is more than enough to demonstrate that the neo Darwinian paradigm is completely inappropriate to explain what we can see in the proteome and in its natural history. And this is only one example among thousands.

So, I want to conclude repeating again this strong and very convinced statement:

The observed facts described here cannot in any way be explained by any neo-darwinian model. Absolutely not. They are extremely strong evidence for a design inference.

Comments
gpuccio- from what I remember Petrushka was fond of equivocating and steadfastly refused to understand what ID was saying.ET
July 25, 2017
July
07
Jul
25
25
2017
05:02 PM
5
05
02
PM
PST
Even with my wildest imagination, I cannot see how that helps the darwinist cause.
Thank god nothing ever gets stuck on a local optima on the fitness landscape where we can see how it was before it become perfected by natural selection.Mung
July 25, 2017
July
07
Jul
25
25
2017
02:52 PM
2
02
52
PM
PST
Answers to wd400: Now, I would like to complete my answers to wd400's statements in his post #133. His last argument there was the following:
Assuming what happened to evolve is the only way a given function could arise (this functional information business) ignores the fact that proteins that have many interactions co-evolve with their interactants.
Again, I don't understand how that can be considered an argument in favor of the neo-darwinian model. It is, indeed, quite the opposite. I thought that I had been clear enough in my OP: "And, as a final note, please consider that these are very complex master regulators, which interact with tens of other complex proteins to effect their functions. The whole system is certainly much more irreducibly complex than we can imagine." Now, if a regulatory protein (and these proteins are indeed master regulators!) performs its function by interacting with a lot of other proteins (as is the case here) the only reasonable conclusion is that the whole regulatory system must be exceedingly irreducibly complex. Because the function (the correct regulation of many important cell processes, in different contexts) can be implemented only if all the "actors", or at least most of them, are present and correctly working and interacting. Now, let's suppose that 10 more proteins must be present and working to cooperate with SATB1 and SATB2 (there are probably more, but just to discuss). wd400 says that our proteins (the SATB proteins) will "co-evolve with their interactants". Whatever that means, it seems that now we have not only 1300+ bits of functional information (and 731 identities) to explain in SATB1 and SATB2, but also a lot of other new functional information that we can find and quantify in the 10 accessory proteins. To get just one regulatory network. Among the many that exist in the cell. Even with my wildest imagination, I cannot see how that helps the darwinist cause. By the way, the essential point of my counter-argument here had already been brilliantly expressed, again, by Origenes in his post #142, in response to wd400. I quote from that: "An important fact that doesn’t sit well with your position. The information jump under discussion is in fact far higher." With this post, I hope that I have completed my "impersonal comments" to wd400's post #133 (a post really remarkable for its ability to summarize in a few lines many of the most frequently used arguments in favor of neo-darwinism). But, after that, wd400 has come back to the discussion with a few other posts, so maybe my verbose inspiration is not yet exhausted... :)gpuccio
July 25, 2017
July
07
Jul
25
25
2017
01:46 PM
1
01
46
PM
PST
ED: If I remember well, he had his (few) ideas, and he was very stubborn about them. But, in general, it was possible to discuss with him for some while.gpuccio
July 25, 2017
July
07
Jul
25
25
2017
01:16 PM
1
01
16
PM
PST
Petruschka has always been a die hard!
A die hard what, is the question.ET
July 25, 2017
July
07
Jul
25
25
2017
12:50 PM
12
12
50
PM
PST
Mung: Petruschka has always been a die hard! :)gpuccio
July 25, 2017
July
07
Jul
25
25
2017
12:22 PM
12
12
22
PM
PST
Do old friends, like Elizabeth, Mark Franck, Petruschka and Zachriel, still post there?
No, No, Yes and No. Even Patrick (aka MathGrrl) has left. Tom English and Joe Felsenstein still post. The list of people I have on ignore there has grown to 14 which probably says about all that needs to be said about it, lol.Mung
July 25, 2017
July
07
Jul
25
25
2017
09:10 AM
9
09
10
AM
PST
Dionisio: You know all about spiders! :) It's thrilling to be at the first place! :) :) It doesn't matter if we accept common descent. We have to accept that natural selection did it, whatever! :) Even us, who don’t understand Neo-Darwinian evolution, whatever it means. :)gpuccio
July 25, 2017
July
07
Jul
25
25
2017
08:21 AM
8
08
21
AM
PST
Mung: How's life at TSZ? Do old friends, like Elizabeth, Mark Franck, Petruschka and Zachriel, still post there?gpuccio
July 25, 2017
July
07
Jul
25
25
2017
08:14 AM
8
08
14
AM
PST
Mung @24:
Apparently if you accept common descent you have to accept that natural selection did it.
Does gpuccio agree with that? :)Dionisio
July 25, 2017
July
07
Jul
25
25
2017
07:56 AM
7
07
56
AM
PST
Interesting how we humans interpret facts differently. For example, about 6 days ago, on July 19, RodW posted a comment @75 saying:
"I have a feeling this thread is dead […]"
On the same day @76 I asked him:
"Why do you have such a feeling? What makes you thing that way?"
I haven't seen RodW's reply yet. But that's fine. I'm used to not getting my questions answered by the politely dissenting interlocutors. A professor complained that my questions are dishonest. Maybe because I used a tricky word ("exactly") in a subliminal way to make it unnoticeable to the politely dissenting interlocutors. Oh, well. :) Now what is interesting is that --contrary to RodW's perception-- this thread was not dead on July 19th. Actually, it doesn't seem dead yet. Here's an interesting piece of simple statistics that shows that the discussion here still goes. Eventually the politely dissenting interlocutors will run out of things to say and the thread will hibernate, though it could remain as a confy corner for friendly chats. But in any case the topic may remain hot for an unforeseeable future.
4 days after RodW's wrong assessment:
July 23, 2017 Popular Posts (Last 30 Days)
[1] Information theory is bad news for Darwin: Evolutionary… (1,299) [2] John Sanford: Darwin a figurehead, not a scientist (1,213) [3] Is Mathematics a Natural Science? (Is that important?) (1,210) [4] Is OOL Part of Darwinian Evolution? (1,208) [5] Interesting proteins: DNA-binding proteins SATB1 and SATB2 (1,039) [9 days since started]
July 24, 2017 Popular Posts (Last 30 Days)
[1] Information theory is bad news for Darwin: Evolutionary… (1,302) [2] Interesting proteins: DNA-binding proteins SATB1 and SATB2 (1,252) [10 days since started] [3] John Sanford: Darwin a figurehead, not a scientist (1,213) [4] Is Mathematics a Natural Science? (Is that important?) (1,210) [5] Is OOL Part of Darwinian Evolution? (1,210)
July 25, 2017 Popular Posts (Last 30 Days)
[1] Interesting proteins: DNA-binding proteins SATB1 and SATB2 (1,306) [11 days since started] [2] Information theory is bad news for Darwin: Evolutionary… (1,302) [3] John Sanford: Darwin a figurehead, not a scientist (1,213) [4] Is OOL Part of Darwinian Evolution? (1,211) [5] Is Mathematics a Natural Science? (Is that important?) (1,210)
Dead thread? :)Dionisio
July 25, 2017
July
07
Jul
25
25
2017
07:46 AM
7
07
46
AM
PST
There is no need to demonstrate that possible intermediates, even if only imagines, could possibly have been naturally selected, even if the theory is based on natural selection.
This is exactly the case in my OP over at TSZ. The author says that natural selection seems to have invented the camera-type eye more than once and claims that a complex eye can evolve from an eye spot in about 360,000 years. His evidence for the former claim is the evidence for common descent. Apparently if you accept common descent you have to accept that natural selection did it.Mung
July 25, 2017
July
07
Jul
25
25
2017
07:45 AM
7
07
45
AM
PST
How strange that there are so many surviving. I supposed neo-darwinain evolution or drift should have reduced them to a few!
Walter ReMine described evolutionary theory as a smorgasbord. I think he nailed it.Mung
July 25, 2017
July
07
Jul
25
25
2017
07:30 AM
7
07
30
AM
PST
gpuccio @167:
As said, it has a significant hit in Parasteatoda tepidariourum (the spider), but no significant hits in drosophila). In the spider, the hit is 83.6 bits, 52% identities. The spider protein is labeled as: “uncharacterized protein LOC107441355”, and is 595 AAs long. I don’t think that much is known about it.
Please, let me disagree with you on this. Much more is known about the spider. Check this out: https://www.youtube.com/embed/IC225eKspGMDionisio
July 25, 2017
July
07
Jul
25
25
2017
05:55 AM
5
05
55
AM
PST
wd400: "This is just silly, of course." OK. It is strange that, while I have written a number of "verbose" and rather detailed comments about your few lines (see posts #144, 149, 157, 159, 171), and you refrained from any comment. But you seem ready to intervene when, in your opinion, I say something "silly". Is it possible that I smell some condescension on your part? :) OK, let's go to your links. While I have not access to the 2017 review, and the abstract is not telling (a good reason for me to abstain from any comment), I have looked at the other 4 links, and I am surprised. With the exception of the first one (an experiment with random sequences in bacteria, that is too vague to mean anything substancial), the other three could have been well quoted by me in support of the reasoning I made in my post #149. Indeed. your link #2 was quoted by me in my post #149! Thank you for adding a couple of new links that support my view that new genes are designed from non coding DNA. You could maybe give a look at my post #149, perhaps even read it, especially the part about NS not applying to the evolution of non coding sequences. And maybe reflect on my real silly statement: The important thing is that neo-darwinism remain unfalsifiable: there is no need to support the theory by molecular intermediates, even if the theory is based on molecular intemrdiates. There is no need to demonstrate that possible intermediates, even if only imagines, could possibly have been naturally selected, even if the theory is based on natural selection. There is no need to show in the lab some real pathway that can build new complex functional information by RV and NS alone, even if the theory is based on the existence of such pathways. Now, I will try to clarify one point that is really important. When I speak of neo-darwinian pathways "that can build new complex functional information by RV and NS alone", and I say that we have none, I mean exactly and literally that: A pathway more or less explicitly demonstrated that can build new complex functional information by RV and natural selection alone. It is no answer to that to: a) show that complex functional information arose in the course of natural history. Of course it arose. My OP here is based on that fact. The problem is: how?. How can we explain that? b) argue that there is some continuity in proteins throughout natural history, in the sense that we can recognize molecular ancestors because some domains are already present before. Of course that is true. I believe in common descent, and in the contituity of proteins, supported by design interventions that add the necessary new functional information. I have fully considered that in my analyisis in the OP here, when I have shown the part of the protein sequence that already has sequence homologies in non vertebrates, I have quantified that information at its highest value (154 bits) and I have subtracted that value fron the total of new functional information generated in the transition to vertebrates. You have not commented at all on my strong statement that complex functions cannot be deconstructed into simple intermediate steps, all of them naturally selectable, each of which needs to be fixed. Let's forget for a moment the of the vanished intermediates. OK, you believe that all of them were conscientiously eaten. We will go back to that point. But what about the deconstruction? Let's go again to the 731 conserved AAs that are detectable for the first time in sharks. So, how do you suggest that we can deconstruct that sequence into simpler, functional, naturally selectable steps? I have reasoned about that in my post #157. And made some quantitative considerations, too. Maybe you could read it. So, what do you suggest? 731 one-aminoacid naturally selectable steps? Each conferring a reproductive advantage? Each selected and fixed in the population? Or rather 182 4 AAs naturally selectable steps? Or do you like it better in twos, or threes, or tens? Or do you believe that neutral drift has a role? If so, I would just remind you that all neutral events are completely random with respect to functional sequence space, and therefore do not change in the least the probability barriers. Which are those we know they are. IOWs, random evolution by neutral variation is completely useless to build complex functional information. You have to rely only on NS, and therefore selectable steps, steps that are fixed in the population because they confer an advantage. That would be showing a neo-darwinian pathway that can build new complex functional information. To identify the intermediates. To explain, and maybe test, if and why they would be naturally selectable. To understand what they are, how many of them exist, how big is the transitition between steps, what probabilistic resources, including evolutionary time, are needed for a realistic random search that can find each candidate to a transition, and for a realistic fixation, given a realistic reproductive advantage (and, possibly, not too much interference from random drift and from Haldane's dilemma). That is science: show examples, facts. Quantify. And, above all, respect the basic principle of science: No theory is good unless and until we support it with good facts. And not, as it often seems to be today: My theory is true because I say so, and unless and until you prove it false beyond any possible doubt!gpuccio
July 25, 2017
July
07
Jul
25
25
2017
05:53 AM
5
05
53
AM
PST
gpuccio,
How strange that there are so many surviving. I supposed neo-darwinain evolution or drift should have reduced them to a few!
There's nothing strange about that. It's just that we don't understand Neo-Darwinian evolution, whatever it means. :)Dionisio
July 25, 2017
July
07
Jul
25
25
2017
05:30 AM
5
05
30
AM
PST
Mung: "The protein family of opsins is very large, with more than 1,000 different opsins having been described so far (Terakita 2005). They fall into different groups (‘subfamilies’) with different functional properties, especially concerning the associated G-protein" How strange that there are so many surviving. I supposed neo-darwinain evolution or drift should have reduced them to a few! :)gpuccio
July 25, 2017
July
07
Jul
25
25
2017
04:35 AM
4
04
35
AM
PST
wd400@
wd400:
Origenes: If huge gaps, like the one between non vertebrates and the first vertebrates (WRT proteins SATB1 and SATB2), are to be expected, why is there no such gap between the whale shark and humans?
I’m not sure you’ve been reading this thread? These genes arose in the ancestors of vertebrates.
You mean 'the missing ancestors', I suppose. Anyway, you claim that huge gaps are to be expected, so here is my question again: why is there no such gap anywhere between the whale shark and humans? Why is it that there is no bad news for Darwinism? Why is it thta smooth intermediates and a total absence of intermediates is explained with equal ease?Origenes
July 25, 2017
July
07
Jul
25
25
2017
02:31 AM
2
02
31
AM
PST
@177 WD400, You commented you already stated info to counter Gpuccio about limitations using BLAST in another post on UD. I was curious and looked through the two links you provide. 1st link, zero reference from you on BLAST. 2nd link, no mentions from you on BLAST. Only Gpuccio mentioned BLAST in first link. Alicia used BLAST in 2nd link, debating Gpuccio. And a few others mentioned Blast, from Dionisio to Me Think. Unless I missed it, search turned up nothing on BLAST by you in the two links your provided. Can you reference a specific comment so I can read why you think BLAST is inappropriate? Or, link it. Or state it here. I'm curious, thanks. You also stated this... "Natural selection removes intermediates, after all." While this OP discusses proteins, do you expect Natural Selection to remove the fossil record as well? Are you advocating Gould's Punctuated Equilibrium?DATCG
July 25, 2017
July
07
Jul
25
25
2017
02:27 AM
2
02
27
AM
PST
wd400: "How old do you think the average disease allele is in human populations? How many do you think we share with chimps? Or elephants? (You don’t even need selection for ancestral variants to die off — drift will do it just fine)." As it seems that you are taking a more active part in the discussion, I will answer some points later, but for the moment just a very simple question: How is it that we can keep 80-90% of junk DNA in our genome, while millions of functional molecular intermediates have simply been cancelled in the course of evolution? Who decides what dies off and what doesn't?gpuccio
July 24, 2017
July
07
Jul
24
24
2017
10:34 PM
10
10
34
PM
PST
Popular Posts (Last 30 Days) Information theory is bad news for Darwin: Evolutionary… (1,302) Interesting proteins: DNA-binding proteins SATB1 and SATB2 (1,252) John Sanford: Darwin a figurehead, not a scientist (1,213) Is Mathematics a Natural Science? (Is that important?) (1,210) Is OOL Part of Darwinian Evolution? (1,210)Dionisio
July 24, 2017
July
07
Jul
24
24
2017
10:02 PM
10
10
02
PM
PST
wd400:
These genes arose in the ancestors of vertebrates.
Question begging.ET
July 24, 2017
July
07
Jul
24
24
2017
07:37 PM
7
07
37
PM
PST
gpuccio, I hope I haven't chosen something that will be a huge time sink for you!
The protein family of opsins is very large, with more than 1,000 different opsins having been described so far (Terakita 2005). They fall into different groups ('subfamilies') with different functional properties, especially concerning the associated G-protein (Terakita 2005). - Andreas Schmidt-Rhaesa. The Evolution of Organ Systems (Oxford Biology)
Mung
July 24, 2017
July
07
Jul
24
24
2017
07:08 PM
7
07
08
PM
PST
The important thing is that neo-darwinism remain unfalsifiable: there is no need to support the theory by molecular intermediates, even if the theory is based on molecular intemrdiates. There is no need to demonstrate that possible intermediates, even if only imagines, could possibly have been naturally selected, even if the theory is based on natural selection. There is no need to show in the lab some real pathway that can build new complex functional information by RV and NS alone, even if the theory is based on the existence of such pathways. No need at all to discuss with those who do not believe in the theory. The truth is where it is, how dare anyone doubt it?
This is just silly, of course. There are plenty of cases where we can reconstruct ancient proteins, and even measure their function (review here for an e.g.). But in cases where a gene arises in a relatively long inter-node in a tree those methods will not work. Instead, we can look a the constituent parts of the gene (in this case containing motifs that exist across the animal tree) and we can to look at more modern genes to understand the processes that contribute the origin of new genes and their early evolution. That's a very rich field of research at present. Here are a couple of relevant papers (1, 2, 3,4), there are many more for anyone that is interested.wd400
July 24, 2017
July
07
Jul
24
24
2017
05:50 PM
5
05
50
PM
PST
But we have to believe that the intermediates existed, if he says so.
You simply have to love a theory that wipes out the evidence that would support it. If we claimed that goddidit, but wiped out his tracks, we'd be laughed at. Goddidit but made it look like evolution is one of my personal favorites. But I don't really believe wd400, because nothing is there to prevent gene duplication so that one gene can evolve into the new form while the other remains. That the evidence got wiped out is just too ad hoc and self-serving.Mung
July 24, 2017
July
07
Jul
24
24
2017
04:52 PM
4
04
52
PM
PST
gpuccio @182:
But we have to believe that the intermediates existed, if he says so.
Of course! it's all a matter of faith. No discussions allowed. Also, it's obvious that we don't understand evolution, whatever that means. :)Dionisio
July 24, 2017
July
07
Jul
24
24
2017
04:43 PM
4
04
43
PM
PST
gpuccio @179:
After all, my posts are “verbose”, so it’s all my fault!
Please, keep them as verbose as you can. Thanks!Dionisio
July 24, 2017
July
07
Jul
24
24
2017
04:22 PM
4
04
22
PM
PST
How can you explain that a lot of apparently normal people harbor genes that favor specific tumors, or thrombosis, and so on? And yet we should believe that hundreds, thousand, maybe millions of molecular intermediates, all of them perfectly functional, so much so that they have been positively selected in the course of natural history, completely disappeared without leaving any trace of themselves?
How old do you think the average disease allele is in human populations? How many do you think we share with chimps? Or elephants? (You don't even need selection for ancestral variatns to die off -- drift will do it just fine).wd400
July 24, 2017
July
07
Jul
24
24
2017
03:52 PM
3
03
52
PM
PST
If huge gaps, like the one between non vertebrates and the first vertebrates (WRT proteins SATB1 and SATB2), are to be expected, why is there no such gap between the whale shark and humans?
I'm not sure you've been reading this thread? These genes arose in the ancestors of vertebrates.wd400
July 24, 2017
July
07
Jul
24
24
2017
03:49 PM
3
03
49
PM
PST
Origenes: Of course, small gradual gaps are expected in neo-darwinian theory. Not at all, IMO, such huge gaps of hundreds of bits as have been shown in my OPs and comments. That's why science has to be quantitative, and not only rely on just so stories supported by dogmatic consensus. You are perfectly correct, if gaps are to be expected, why do we see them only at certain crucial passages, and much more in some proteins than in others? Regarding the "branching nature" of evolutionary process, he is again arguing against his same theory. A perfect cancellation of all the intermediate forms requires that each step is completely fixed, and that all alternative forms of the functional protein, those same alternative forms that had been fixed in the previous step, are completely cancelled. But the proteins that existed in non vertebrates are not cancelled by those that we find in vertebrates. Even today, in the human proteome, a lot of polymorphisms exist, some of them even certainly deleterious. How can you explain that a lot of apparently normal people harbor genes that favor specific tumors, or thrombosis, and so on? And yet we should believe that hundreds, thousand, maybe millions of molecular intermediates, all of them perfectly functional, so much so that they have been positively selected in the course of natural history, completely disappeared without leaving any trace of themselves? The important thing is that neo-darwinism remain unfalsifiable: there is no need to support the theory by molecular intermediates, even if the theory is based on molecular intemrdiates. There is no need to demonstrate that possible intermediates, even if only imagines, could possibly have been naturally selected, even if the theory is based on natural selection. There is no need to show in the lab some real pathway that can build new complex functional information by RV and NS alone, even if the theory is based on the existence of such pathways. No need at all to discuss with those who do not believe in the theory. The truth is where it is, how dare anyone doubt it?gpuccio
July 24, 2017
July
07
Jul
24
24
2017
03:44 PM
3
03
44
PM
PST
1 2 3 4 5 6 … 11